The Invisible Gradient: Why Oxygen Distribution Might Be the Real Difference Between Good and Great Trichoderma
The green carpet on our SSF trays is beautiful, no doubt. But if you look past the colour and focus on what the fungus is actually breathing, a far more interesting story unfolds.
We talk a lot about moisture, temperature, and substrate composition. But there is another parameter—silent, invisible, and arguably more decisive—that separates a mediocre batch from a biochemically potent one. That parameter is oxygen.
And here is the twist: how oxygen reaches Trichoderma in Solid-State Fermentation (SSF) is fundamentally different from how it works in Submerged Fermentation (SmF). Understanding this difference isn't just academic trivia. It explains why SSF produces spores that are biochemically primed for the monsoon—and why the oxygen gradient within our trays might be the secret ingredient we have been overlooking.
The SmF Oxygen Reality: Homogeneous but Demanding
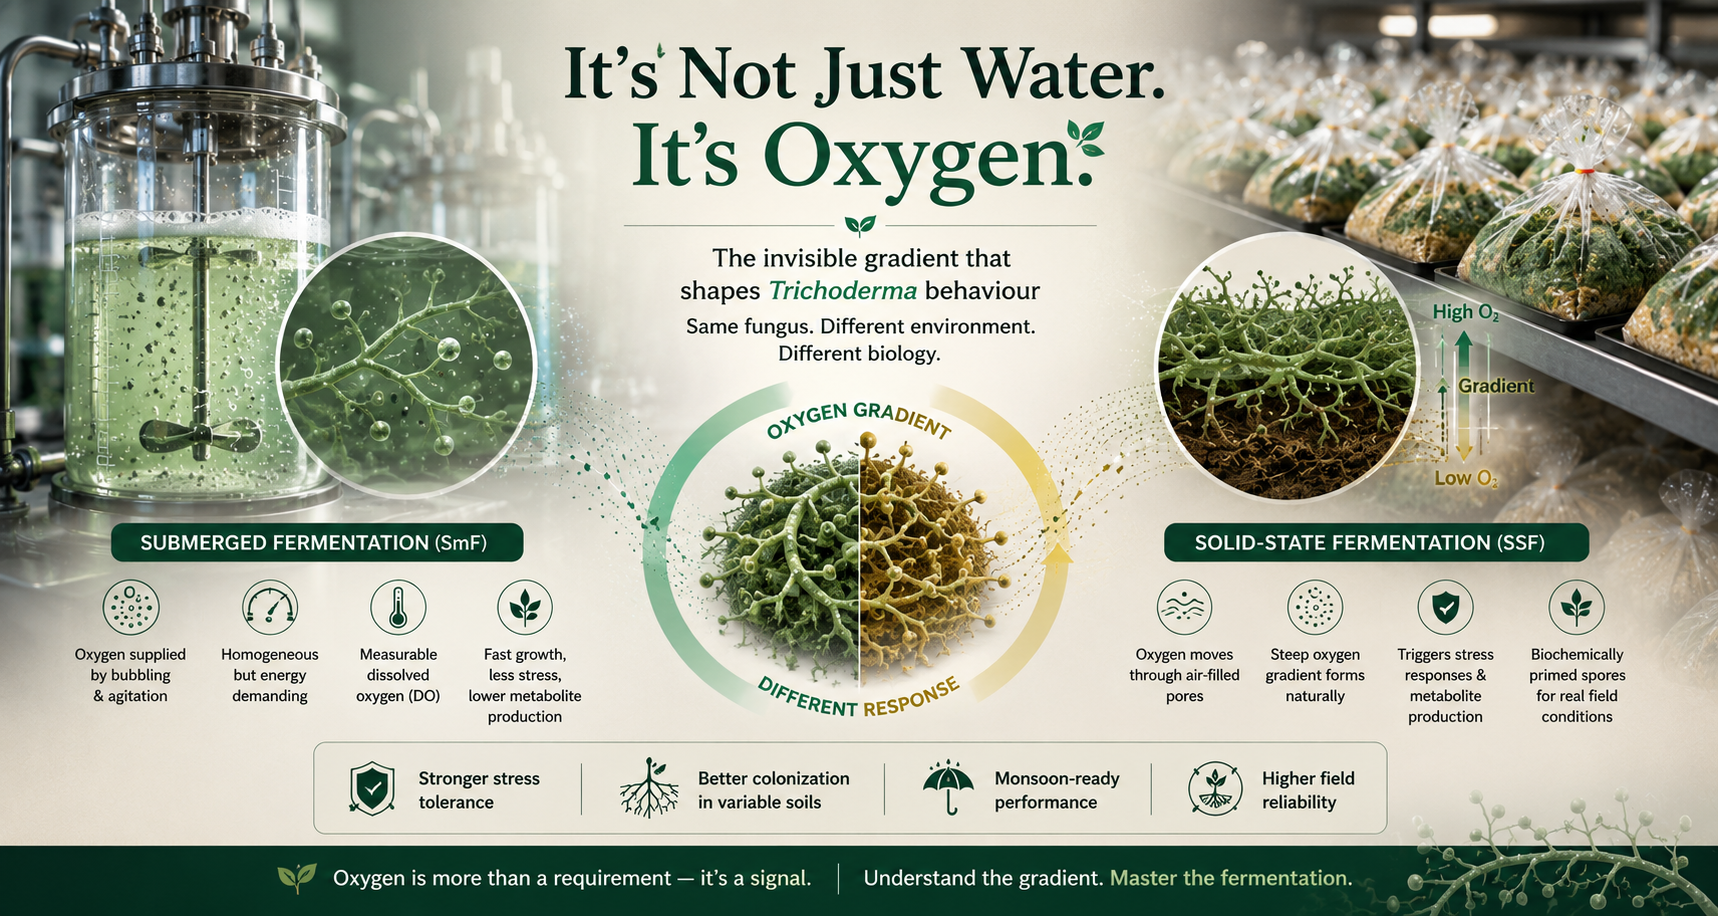
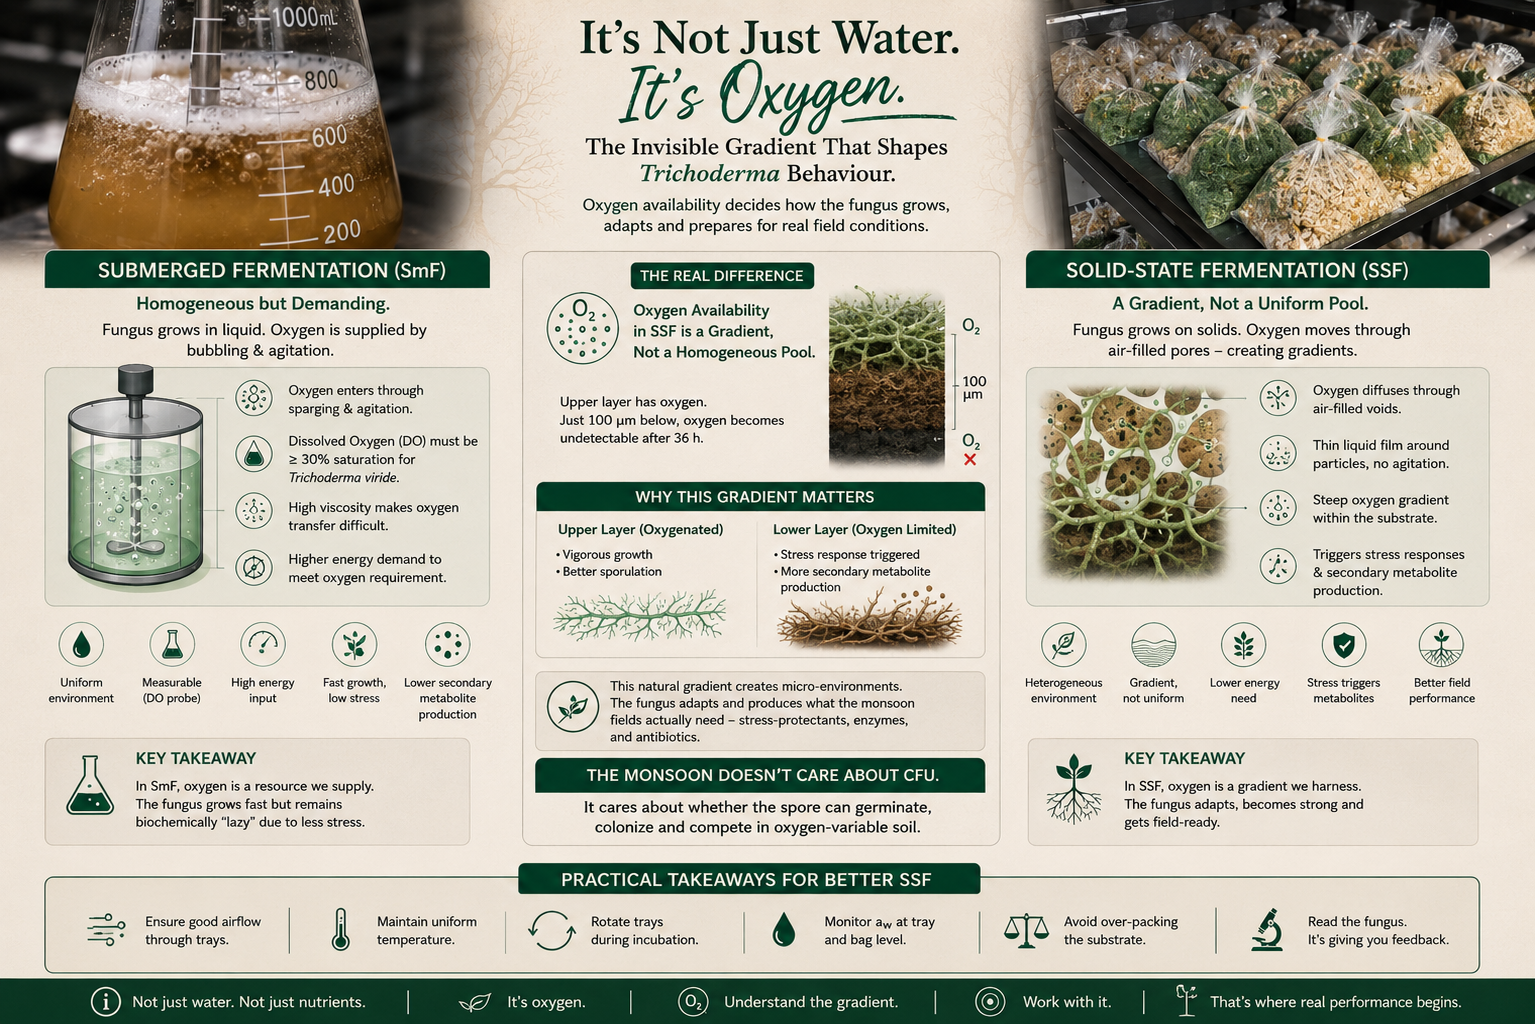
In submerged fermentation, Trichoderma grows in a liquid broth—water, sugars, nutrients, all mixed together. Oxygen enters the system through sparging (bubbling air) and mechanical agitation. The gas bubbles diffuse into the liquid, dissolve at the gas-liquid interface, and then travel through the bulk liquid to reach the fungus.
This setup is relatively predictable. Dissolved oxygen (DO) concentration can be measured with a probe. The volumetric oxygen mass transfer coefficient is a standard parameter that engineers track closely.
For Trichoderma viride, maintaining dissolved oxygen at or above 30% saturation is critical for growth and conidia production. Drop below that, and the fungus struggles.
But here is the catch: Trichoderma is a filamentous fungus. As it grows, it develops hyphae, creating a highly viscous, shear-thinning medium. This viscosity makes oxygen transfer increasingly difficult. To keep up with the oxygen demand, agitation and aeration requirements escalate significantly, especially at higher biomass concentrations. The system becomes energy-intensive and technically demanding.
The SSF Oxygen Reality: A Gradient, Not a Homogeneous Pool
Now, shift your gaze to our SSF trays. The fungus grows on the surface of solid particles—rice bran, wheat straw—surrounded by a thin liquid film and air-filled void spaces. The water content is low, typically around 55–60%. There is no bulk liquid. There are no bubbles. There is no mechanical agitation.
So, how does oxygen reach the fungus?
Here is the counterintuitive part: oxygen mass transfer is actually more efficient in SSF than in SmF—on paper, at least. Why? Because the fungus is in close contact with the gaseous oxygen that flows through the void spaces between solid particles. The higher area-to-volume ratio of the solid matrix facilitates oxygen transfer. In theory, oxygen is everywhere.
But "everywhere" is not the same as "available."
In reality, SSF creates steep oxygen concentration gradients. The fungal mat itself develops into layers—an upper layer of sparse aerial hyphae with gas-filled pores, and a dense bottom layer with liquid-filled pores. Oxygen microelectrode measurements have shown that while the upper aerial layer remains oxygenated, oxygen becomes undetectable just 100 micrometres below the gas-liquid interface after 36 hours of cultivation.
Let that sink in. One hundred micrometres. That is thinner than a human hair. And yet, oxygen cannot penetrate beyond that depth.
The consequence? The fungus in the deeper, wetter layers experiences oxygen depletion. And when oxygen is limited, Trichoderma viride shifts its metabolism. It switches to a fermentative pathway, producing ethanol, succinate, and other carboxylic acids. The appearance of secondary metabolites is directly modified by oxygen availability.
Why This Gradient Matters for Your SSF Trays
This oxygen gradient is not a problem to be solved. It is a feature—and perhaps the very reason SSF produces such potent biocontrol agents.
The gradient creates microenvironments within a single tray. The upper layers, bathed in oxygen, support vigorous growth and sporulation. The deeper layers, oxygen-limited, trigger stress responses that upregulate secondary metabolite production. The fungus is not a uniform mass; it is a heterogeneous population responding to local conditions. And heterogeneity, in this context, might be a good thing.
The Practical Takeaway
- In SmF, oxygen is a resource you must constantly supply. It is homogeneous, measurable, and energy-intensive to maintain. The fungus grows fast but biochemically "lazy" because stress is minimised.
- In SSF, oxygen is a gradient. It is heterogeneous, self-organising, and creates natural stress zones within the substrate. The fungus adapts—producing stress-protectants, antibiotics, and enzymes in response to local oxygen depletion.
The monsoon doesn't care about your CFU count. It cares about whether the spore can germinate, colonise, and compete in oxygen-variable soil conditions. And that readiness? It is forged in the oxygen gradients of your SSF trays.
The question that lingers:
Are we still treating oxygen as a simple "supply" problem—or are we ready to embrace the gradient as a deliberate tool for biochemical conditioning?
Our trays have been telling us this story all along. It is time we started listening.
What the Green on Our Trays Is Really Telling Us
The lab has that distinct smell again. Earthy, slightly sweet, with a ghost of coconut lingering near the incubation racks. That’s 6-pentyl-α-pyrone off-gassing from our Solid-State Fermentation trays.
Monsoon is almost here. And if you look past the sales charts and the farmer helplines buzzing in the background, what we’re actually doing in this room is far more fascinating than just scaling up a biopesticide.
We are forcing a microscopic organism to make a life-or-death biochemical decision.
Walk through our production floor, and you will see the trays. Stacked high. Filled with agricultural waste—rice bran, wheat straw —all knitted together by that unmistakable green mycelial mat. Visitors usually ask about the "yield." How many spores per gram? What’s the CFU count?
I used to ask those questions too. But lately, I have started asking a different one: What exactly are we harvesting?
If you compare this to liquid fermentation, the difference is staggering.
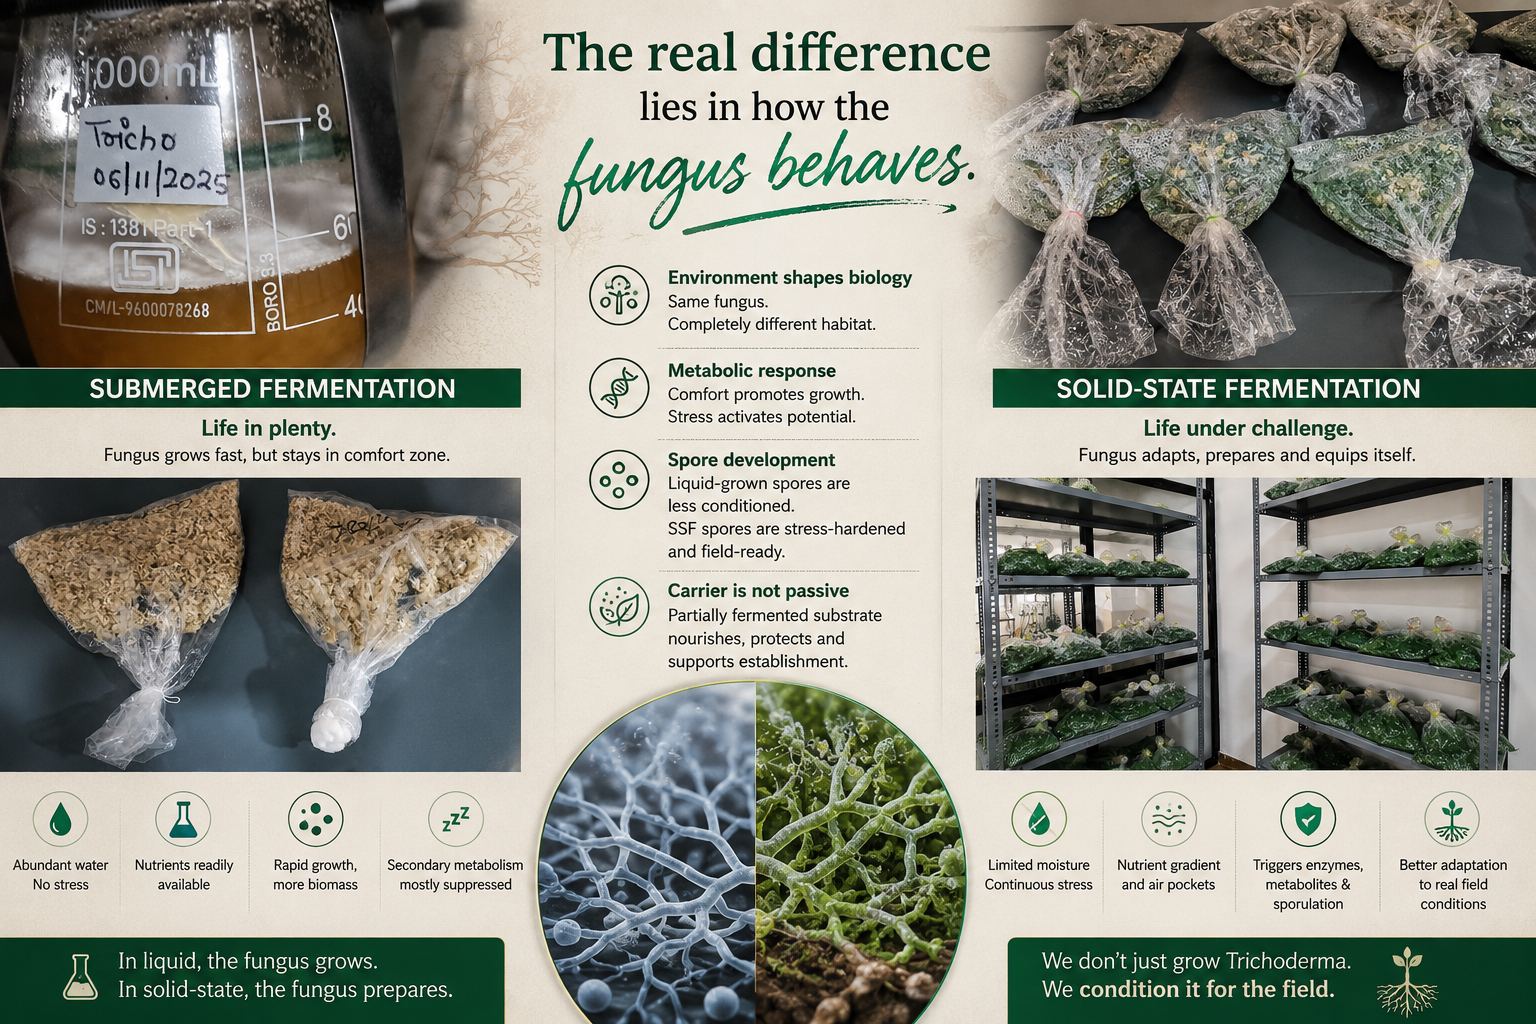
In a liquid broth, Trichoderma lives like a spoiled child. Unlimited water, abundant dissolved sugars, constant agitation. It grows fast, sure. But biochemically? It gets lazy.
The genes responsible for producing its chemical weapons—the polyketides, the peptaibols, the volatile antibiotics—mostly stay switched off. Why fire a missile when there is no war?
Solid-state fermentation flips that comfort zone upside down.
The moment we mix the substrate to that narrow sweet spot of 55-60% moisture, we create a physical paradox for the fungus. It is surrounded by solid particles, air pockets, and just enough water to survive, but not enough to thrive without effort.
The low water activity and the gradient of nutrients across the solid matrix act as a constant, low-level stress signal.
And stress, as every biochemist knows, is the greatest catalyst for secondary metabolism.
Under this subtle pressure, Trichoderma wakes up. It ramps up its non-ribosomal peptide synthetases.
It starts pumping out chitinases and glucanases, not just into a diluted liquid medium, but right into the micro-pores of the substrate where they concentrate to remarkably high local levels.
When that spore eventually lands in a waterlogged paddy field, it doesn't start from scratch. It carries those pre-formed enzymes with it, like a soldier carrying a loaded weapon to the frontline. The pathogen doesn't stand a chance.
There is another layer to this that doesn't get enough attention—the biochemistry of the spore itself.
Spores harvested from SSF trays are not the same as those washed out of a bioreactor.
Under the low-water stress of solid substrates, the fungus accumulates protective solutes like trehalose and mannitol. These are nature’s antifreeze and desiccation protectants.
Monsoon soils are brutal—they swing from saturated to dry and back again within days.
A liquid-cultured spore, with its thinner biochemical armor, often gets caught off guard. But an SSF-matured spore? It has already survived the harshest conditions of the production floor. It is biochemically primed to germinate aggressively the moment it senses root exudates.
And I haven't even mentioned the carrier yet.
We tend to think of the spent substrate as just that—spent. Inert. A vehicle to get the spores from our lab to the field. But that partially fermented agricultural waste is a biochemical time-release capsule. It is loaded with residual reducing sugars, organic acids, and even some of the very volatile organic compounds that Trichoderma uses to communicate with plant roots.
When the farmer mixes this powder with water and applies it to the soil, that carrier doesn't just dissolve away. It feeds the germinating spores, gives them a head start, and acts as a prebiotic cushion in the rhizosphere.
So, standing here with a tray in my hands, looking at the dense green sporulation, I no longer see a "mass multiplication unit." I see a miniature biochemical reactor where nature’s most sophisticated fungal agent is forced to reveal its full arsenal.
We are not growing Trichoderma here. We are negotiating with it. We provide the physical stress, the solid matrix, the imperfect environment—and in exchange, it gives us everything it has. The antibiotics. The lytic enzymes. The stress-protectants. The signaling molecules. All compressed into that green powder.
The monsoon doesn't make this product sell. The monsoon simply wakes up the biochemistry that we have already drawn out out of the fungus, weeks in advance, right there on those trays.
The question that keeps me up at night is this: Are we still evaluating our product purely by the number of green dots on a hemocytometer? Or are we finally ready to measure what actually matters—the biochemical maturity of every single spore we send out the door? Because looking at these trays, I think the fungus has already made its choice. It’s time we made ours.